Can Astaxanthin Support Mitochondrial Resilience?
Keyora Research Q&A Library
This is part of the Keyora Research Q&A Series, derived from Keyora Astaxanthin Research Journal Series.
Within the Keyora Astaxanthin Researcn framework, this Q&A translates complex astaxanthin biology into reader-friendly, evidence-bound answers, focusing on natural astaxanthin identity, molecular structure, antioxidant and redox mechanisms, membrane lipid interaction, mitochondrial resilience, inflammatory signaling pathways, human evidence interpretation, and the scientific principles behind responsible supplementation.
First published by Keyora Research Journal: www.keyorahealth.com
Direct Answer
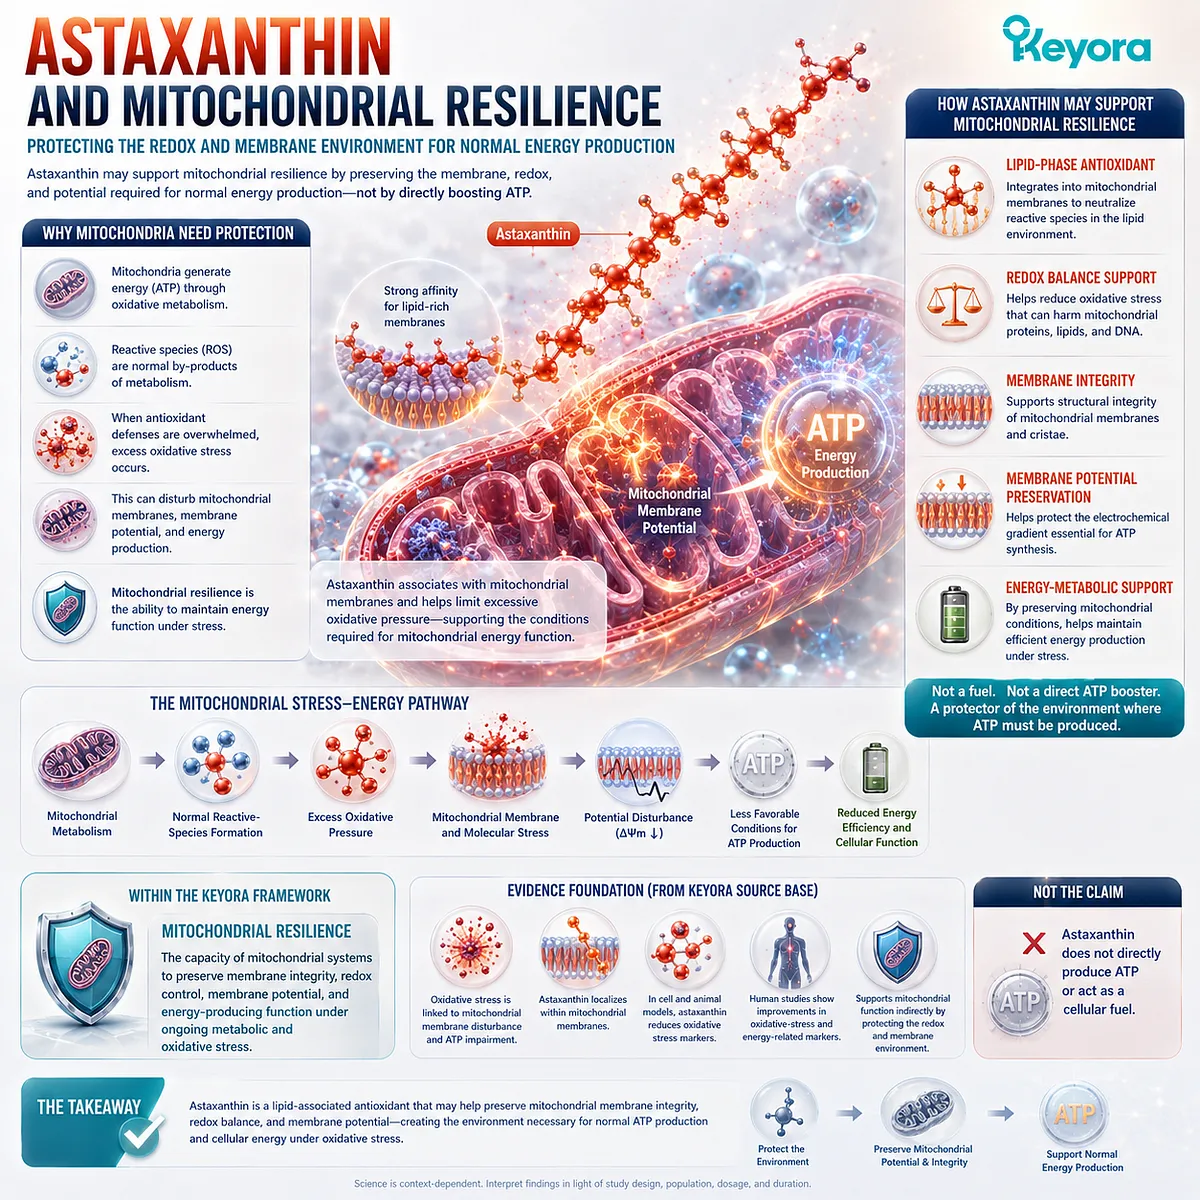
Astaxanthin may support mitochondrial resilience by protecting the redox and membrane environment required for normal energy production
Astaxanthin may support mitochondrial resilience, but the most scientifically appropriate interpretation is not that it directly “boosts ATP” or acts as a cellular fuel.
Its relevance comes from the relationship between oxidative stress, mitochondrial membranes, membrane potential, and the conditions required for normal energy production.
The Keyora source base repeatedly connects excessive oxidative stress with mitochondrial membrane disturbance and impaired ATP-related function.
In one section, oxidative stress is described as disrupting mitochondrial membrane potential and ATP production, illustrating why mitochondrial energy metabolism cannot be separated from mitochondrial redox balance.
The core pathway is therefore:
Mitochondrial metabolism
↓
Normal reactive-species formation
↓
Excess oxidative pressure when regulation is overwhelmed
↓
Mitochondrial membrane and molecular stress
↓
Potential disturbance of membrane potential
↓
Less favorable conditions for ATP production
Astaxanthin enters this pathway as an antioxidant with strong affinity for lipid-rich biological environments.
Within the Keyora framework, Mitochondrial Resilience can be defined as:
the capacity of mitochondrial systems to preserve membrane integrity, redox control, membrane potential, and energy-producing function under ongoing metabolic and oxidative stress
Astaxanthin may support that resilience by helping limit excessive oxidative pressure around mitochondrial structures.
That is different from saying Astaxanthin itself generates ATP.
It is better understood as helping preserve the environment in which mitochondrial energy production must operate.
Why Are Mitochondria Especially Exposed to Oxidative Stress?
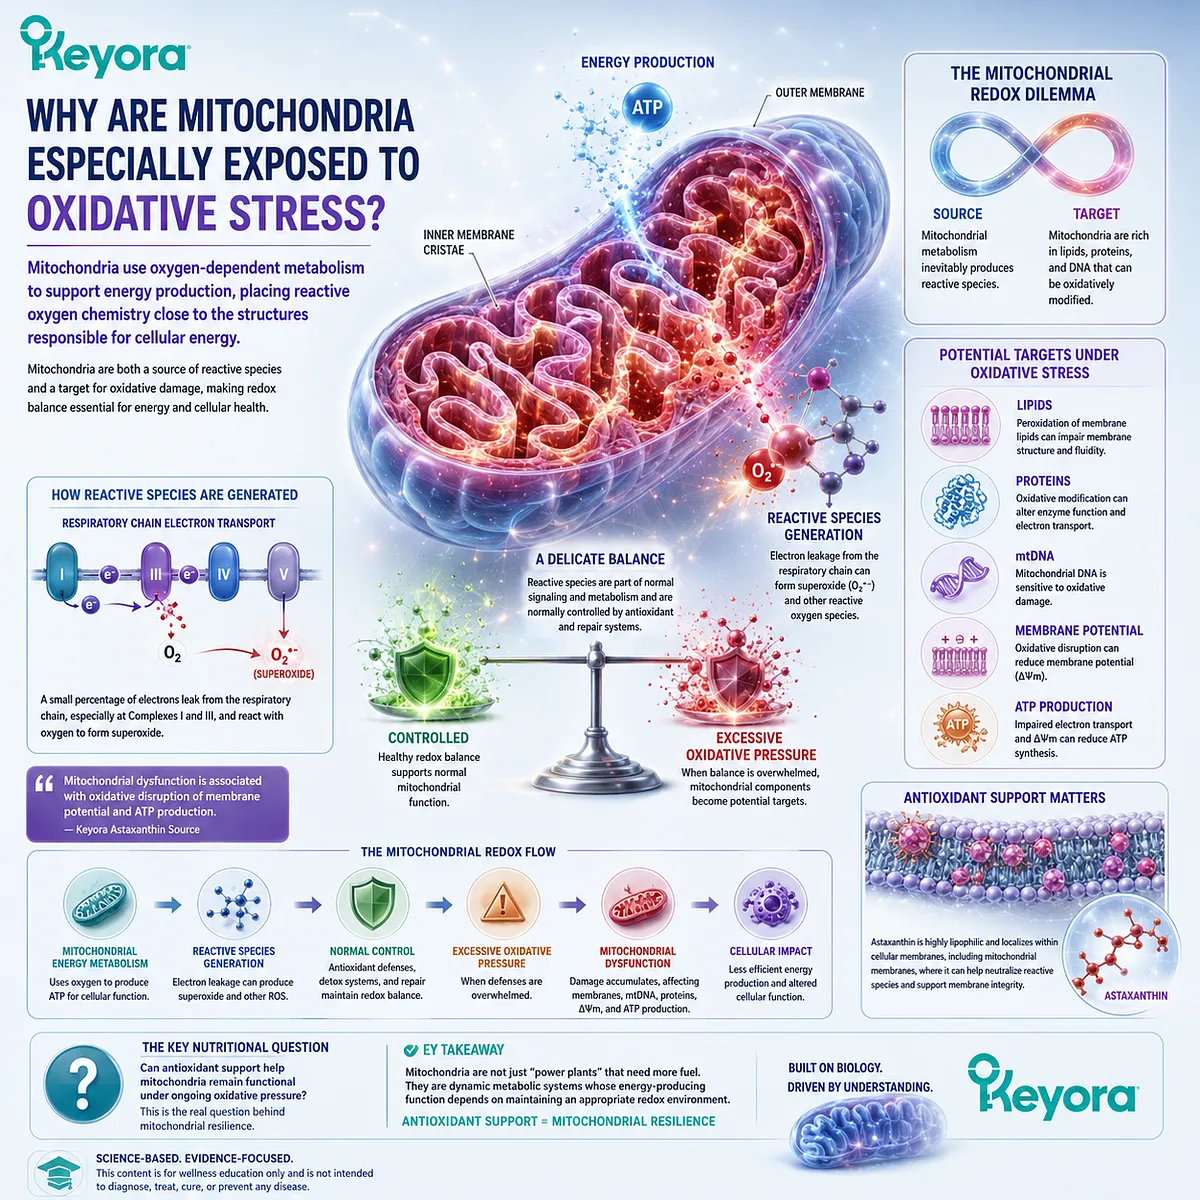
Mitochondria use oxygen-dependent metabolism to support energy production, placing reactive oxygen chemistry close to the structures responsible for cellular energy
Mitochondria occupy an unusual position in redox biology because they are both involved in the production of reactive oxygen species and vulnerable to excessive oxidative stress.
The Keyora Astaxanthin source lists mitochondrial energy metabolism as an endogenous source of reactive species. It specifically describes electron leakage from the respiratory chain as a source of superoxide formation.
That does not mean normal mitochondrial metabolism is inherently damaging.
Reactive oxygen species are also part of normal cellular signaling and metabolism. The biological problem arises when reactive-species generation exceeds the capacity of antioxidant, detoxification, repair, and turnover systems to maintain redox balance.
This creates an important dual relationship:
Mitochondria produce energy
↓
Energy metabolism can generate reactive species
↓
Reactive species are normally controlled
but under excessive oxidative pressure:
Mitochondrial lipids, proteins, and membranes become potential oxidative targets
The Keyora source also associates mitochondrial dysfunction with oxidative disruption of membrane potential and ATP production.
This is why mitochondria are frequently discussed in antioxidant research.
They are not simply “power plants” that need more fuel.
They are dynamic metabolic systems whose energy-producing function depends on maintaining an appropriate redox environment.
From the Keyora perspective, the relevant nutritional question therefore becomes:
Can antioxidant support help mitochondria remain functional under ongoing oxidative pressure?
For Astaxanthin, this question is particularly relevant because its antioxidant activity is closely associated with lipid-rich membrane environments.
Why Does the Mitochondrial Membrane Matter for ATP Production?
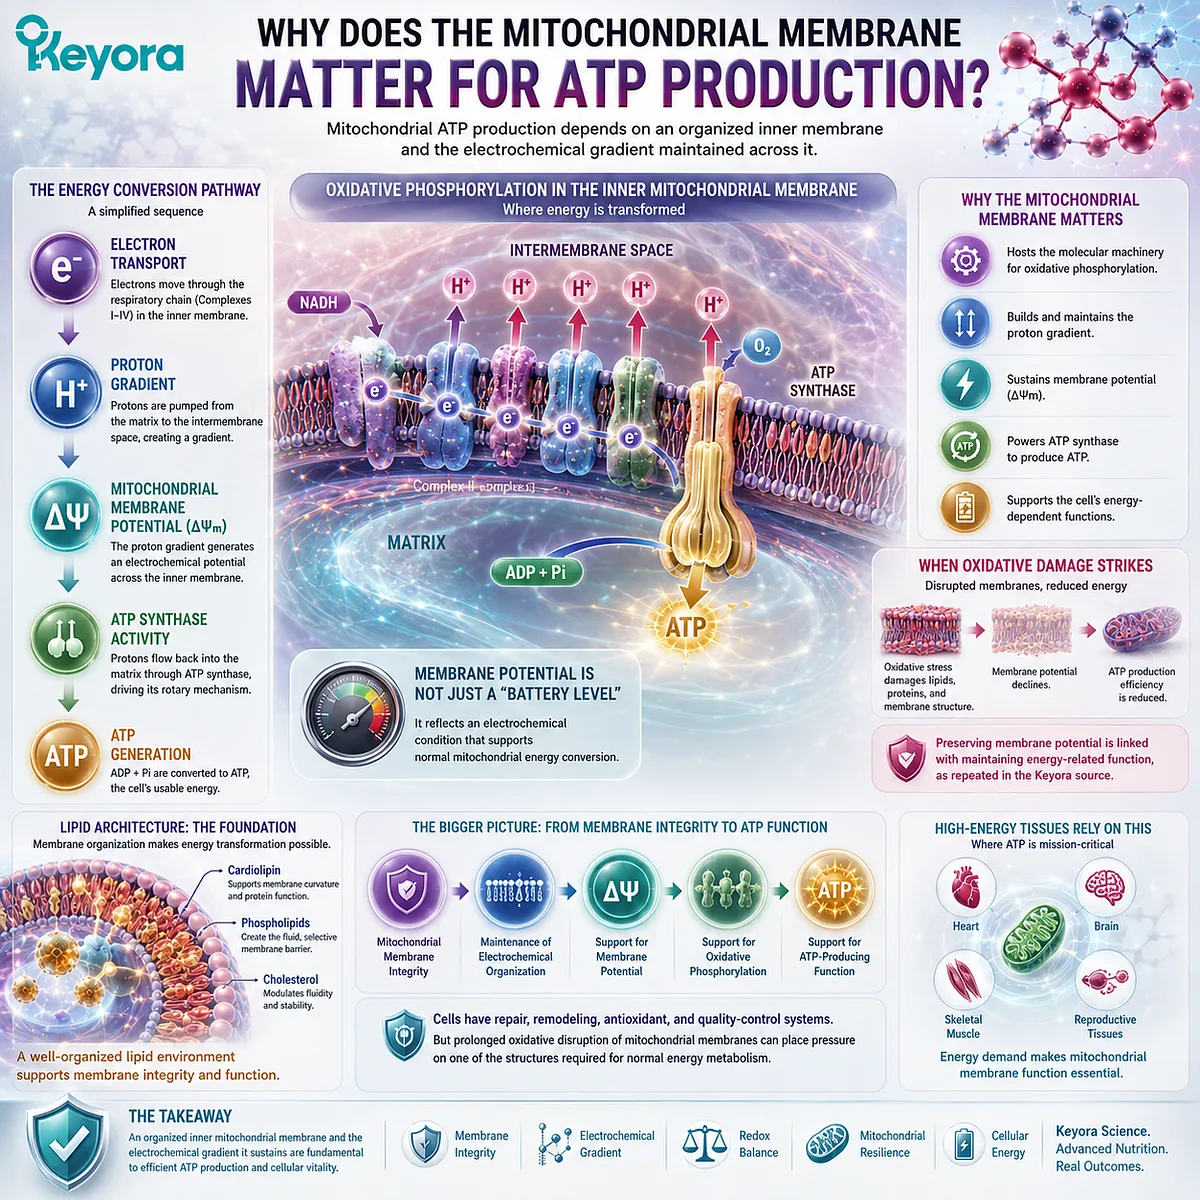
Mitochondrial ATP production depends on an organized inner membrane and the electrochemical gradient maintained across it
Mitochondrial energy production is inseparable from membrane architecture.
The inner mitochondrial membrane contains the molecular machinery involved in oxidative phosphorylation. Electron-transfer processes help establish an electrochemical gradient across this membrane, and that gradient provides the driving force used by ATP synthase to generate ATP.
A simplified pathway is:
Electron transport
↓
Proton gradient
↓
Mitochondrial membrane potential
↓
ATP synthase activity
↓
ATP generation
This is why mitochondrial membrane potential is such an important concept.
It should not be imagined simply as a “battery level.”
Rather, membrane potential reflects an electrochemical condition that supports normal mitochondrial energy conversion.
The Keyora source repeatedly places membrane potential and ATP production in the same mechanistic framework. In reproductive tissue discussions, it describes oxidative damage as impairing mitochondrial membranes and reducing ATP production efficiency, while preservation of membrane potential is linked with maintenance of energy-related function.
This extends the Lipid Architecture concept developed earlier in the Q&A series.
Membranes are not only boundaries around cells.
They are also functional platforms inside cells.
In mitochondria, membrane organization helps make energy transformation possible.
The important sequence is therefore:
Mitochondrial membrane integrity
↓
maintenance of electrochemical organization
↓
support for membrane potential
↓
support for oxidative phosphorylation
↓
support for ATP-producing function
This does not mean every change in mitochondrial membrane chemistry immediately causes energy failure.
Cells possess multiple repair, remodeling, antioxidant, and quality-control systems.
But it does mean that prolonged oxidative disruption of mitochondrial membranes can place pressure on one of the structures required for normal energy metabolism.
How Can Oxidative Stress Disrupt Mitochondrial Energy Production?
Excess oxidative stress can modify mitochondrial lipids and proteins, increasing the burden on the membrane systems that support energy production
Mitochondrial oxidative stress matters because the structures involved in energy production are themselves chemically vulnerable.
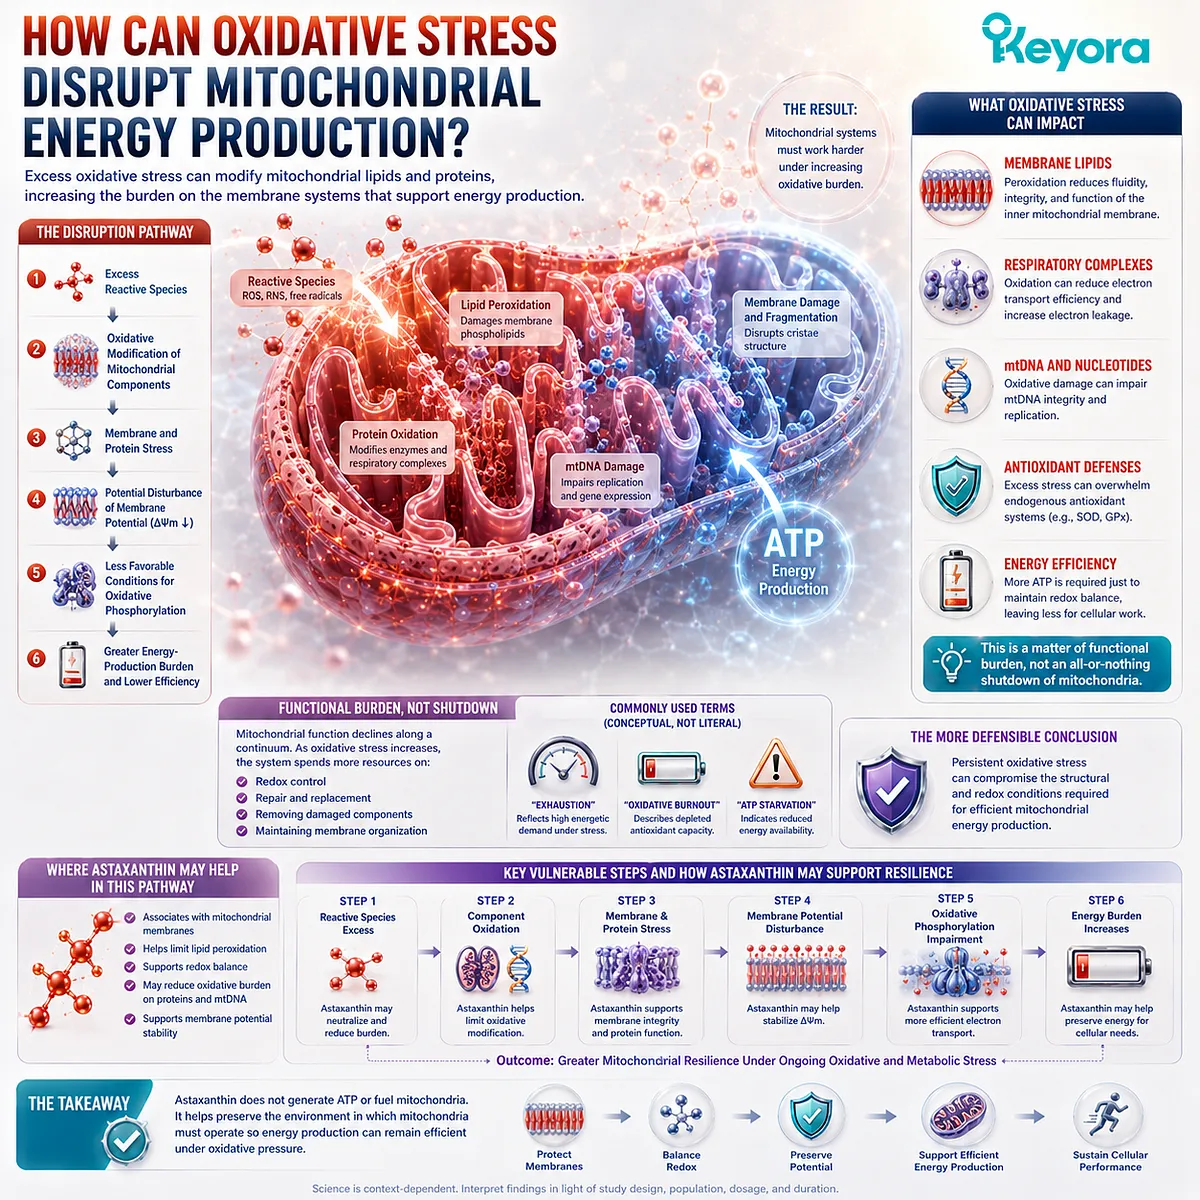
Persistent oxidative pressure can modify membrane lipids, proteins, and other mitochondrial components. When those changes accumulate faster than repair and turnover systems can manage them, mitochondrial function may become less efficient.
The Keyora source describes this relationship in several tissue contexts. It links oxidative damage with impaired mitochondrial membrane integrity, reduced membrane potential, and less efficient ATP production.
The biological pathway can be simplified as:
Excess reactive species
↓
Oxidative modification of mitochondrial components
↓
Membrane and protein stress
↓
Potential disturbance of membrane potential
↓
Less favorable conditions for oxidative phosphorylation
↓
Greater energy-production burden
This is more precise than saying:
“Oxidative stress shuts down mitochondria.”
Mitochondrial function is not usually an all-or-nothing state.
A more accurate concept is functional burden.
As oxidative stress increases, mitochondrial systems may need to devote more resources to maintaining redox control, replacing damaged components, and preserving membrane organization.
The source material sometimes uses stronger terms such as mitochondrial “exhaustion,” “oxidative burnout,” and “ATP starvation” when discussing the energetic demands of the heart.
For public scientific interpretation, those phrases are better treated as conceptual metaphors rather than literal universal physiological states.
The more defensible conclusion is:
Persistent oxidative stress can compromise the structural and redox conditions required for efficient mitochondrial energy production.
That is the problem Astaxanthin mitochondrial research attempts to address.
Can Mitochondrial Oxidative Stress Become a Feedback Loop?
When oxidative pressure compromises mitochondrial function, the same energy-producing system may become less effective at maintaining redox stability
Mitochondrial oxidative stress can become biologically important because the relationship between energy metabolism and redox balance can operate in both directions.
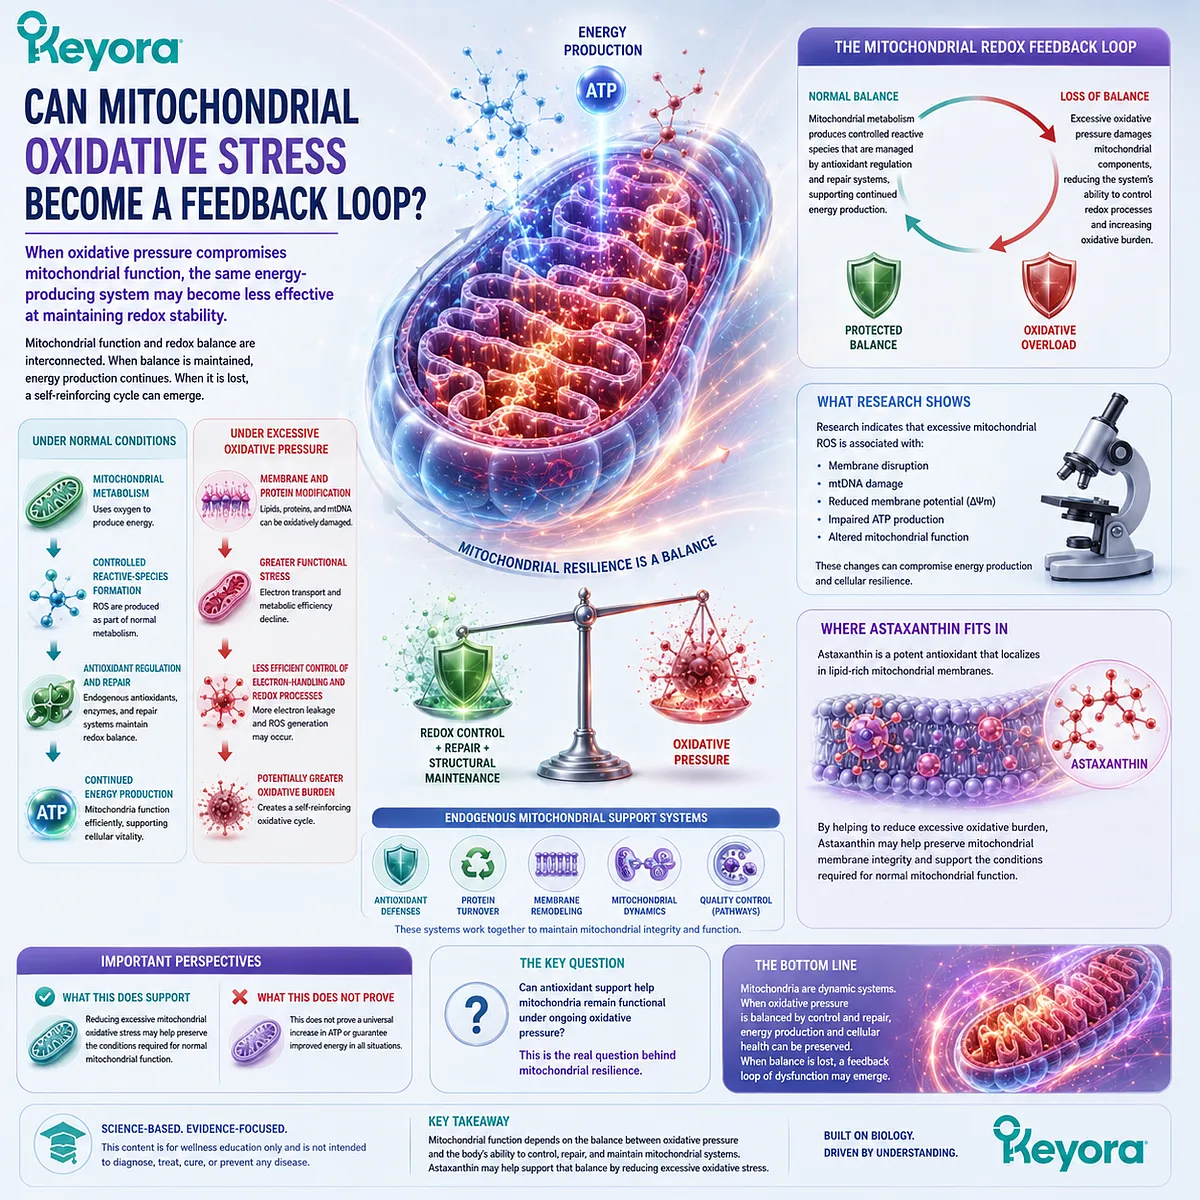
Under normal conditions:
Mitochondrial metabolism
↓
controlled reactive-species formation
↓
antioxidant regulation and repair
↓
continued energy production
But if oxidative pressure becomes excessive:
Membrane and protein modification
↓
greater functional stress
↓
less efficient control of electron-handling and redox processes
↓
potentially greater oxidative burden
This creates what can be described as a Mitochondrial Redox Feedback problem.
The concept should not be interpreted as an inevitable “death spiral.” Mitochondria are supported by endogenous antioxidant systems, protein turnover, membrane remodeling, mitochondrial dynamics, and quality-control pathways.
The key issue is whether those protective systems can keep pace with oxidative demand.
The Keyora sources repeatedly connect excessive mitochondrial ROS with membrane disruption and compromised energy-related function.
This makes mitochondrial resilience a question of balance:
oxidative pressure
versus
redox control + repair + structural maintenance
Astaxanthin becomes relevant because it may influence one side of that balance – the oxidative burden.
If oxidative damage can be limited, mitochondrial membranes and associated energy-producing machinery may operate in a more favorable biochemical environment.
That does not prove a universal increase in ATP.
It supports a more specific hypothesis:
reducing excessive mitochondrial oxidative stress may help preserve the conditions required for normal mitochondrial function
This distinction keeps Mitochondrial Resilience grounded in biology rather than turning it into a generalized “energy booster” claim.
How Could Astaxanthin Support Mitochondrial Membranes and Redox Balance?
Astaxanthin’s antioxidant and lipid-associated properties provide a plausible mechanism for reducing oxidative pressure around mitochondrial structures
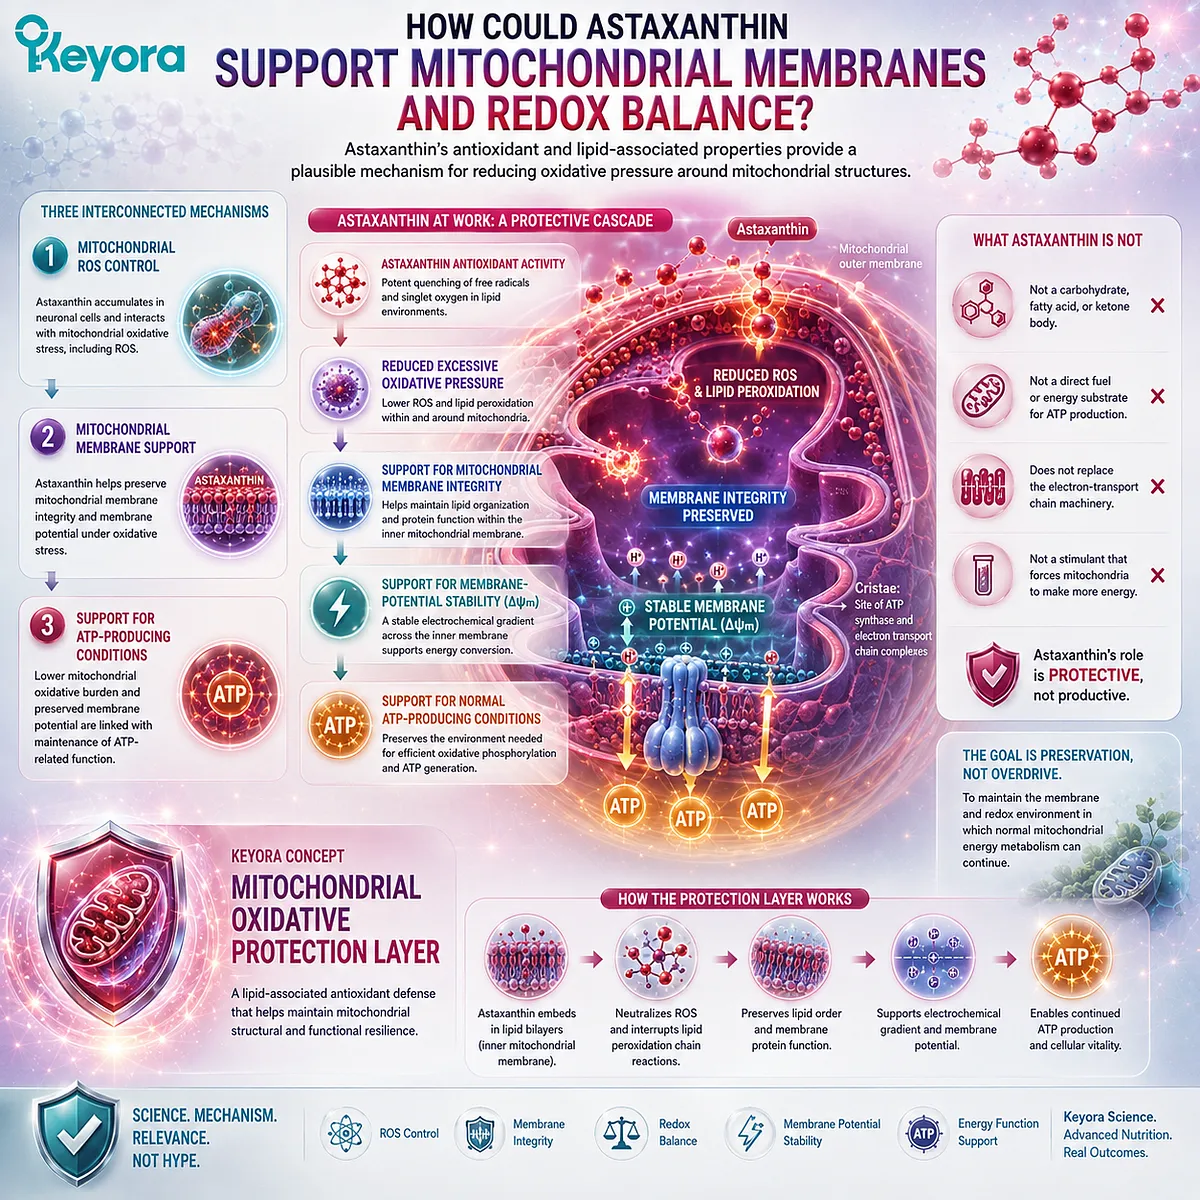
Astaxanthin enters mitochondrial research through three interconnected mechanisms described in the Keyora source base.
First is mitochondrial ROS control.
In neural contexts, the source describes Astaxanthin as accumulating within neuronal cells and interacting with mitochondrial oxidative stress, including mitochondrial ROS.
Second is mitochondrial membrane support.
In reproductive tissue discussions, the source links Astaxanthin with preservation of mitochondrial membrane integrity and membrane potential under oxidative stress.
Third is support for ATP-producing conditions.
The source connects lower mitochondrial oxidative burden and preservation of membrane potential with maintenance of ATP-related function.
Together:
Astaxanthin antioxidant activity
↓
Reduced excessive oxidative pressure
↓
Support for mitochondrial membrane integrity
↓
Support for membrane-potential stability
↓
Support for normal ATP-producing conditions
This sequence is important because it correctly positions Astaxanthin.
Astaxanthin is not a carbohydrate, fatty acid, ketone body, or other metabolic substrate used directly to manufacture ATP.
It also does not replace the electron-transport machinery.
Its proposed role is protective.
A useful Keyora description is:
Mitochondrial Oxidative Protection Layer
The purpose of that layer is not to force mitochondria to produce more energy.
It is to help maintain the membrane and redox environment in which normal mitochondrial energy metabolism can continue.
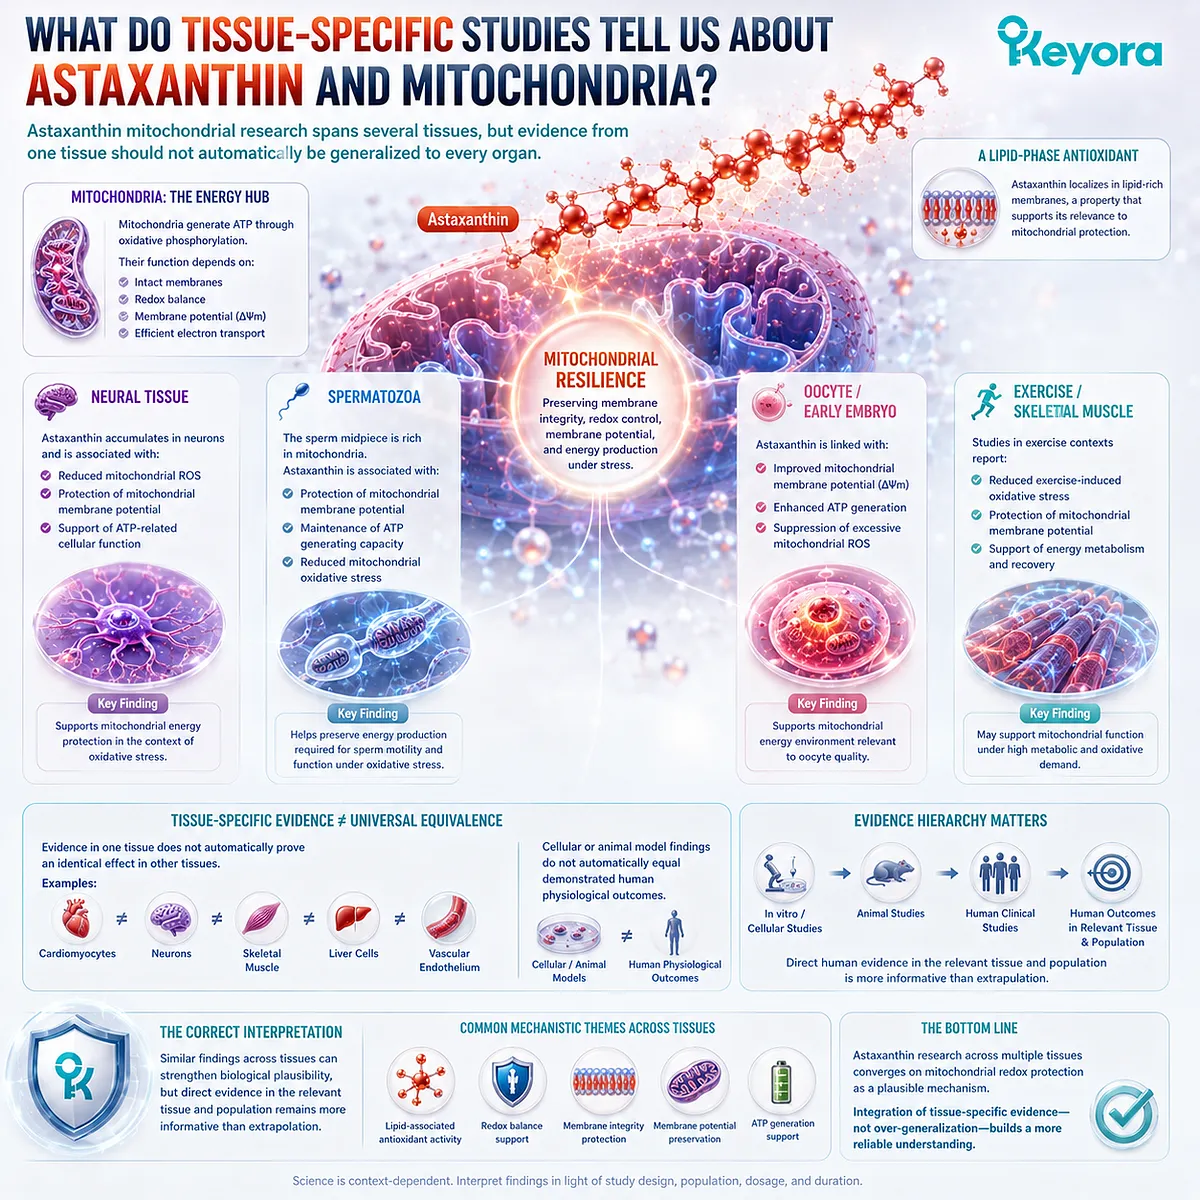
What Do Tissue-Specific Studies Tell Us About Astaxanthin and Mitochondria?
Astaxanthin mitochondrial research spans several tissues, but evidence from one tissue should not automatically be generalized to every organ
The supplied Keyora sources discuss mitochondrial effects across neural, reproductive, and exercise-related contexts.
In neural tissue, Astaxanthin is associated with reduced mitochondrial oxidative stress and protection of energy-related cellular function. The source specifically discusses neuronal accumulation and mitochondrial ROS control.
In sperm biology, the source notes that the sperm midpiece is rich in mitochondria and connects Astaxanthin with protection of ATP-generating capacity under oxidative stress.
In oocyte-related material, the source connects Astaxanthin with mitochondrial membrane potential, ATP generation, and suppression of excessive mitochondrial ROS.
The repeated appearance of similar mechanisms across different biological systems supports an important idea:
mitochondrial oxidative protection is not necessarily confined to one tissue type.
However, tissue-specific evidence must remain tissue-specific.
Evidence in sperm mitochondria does not automatically prove an identical effect in:
-
cardiomyocytes;
-
neurons;
-
skeletal muscle;
-
liver cells;
-
vascular endothelium.
Likewise, findings in cellular or animal models should not automatically be presented as demonstrated human physiological outcomes.
The correct interpretation is:
similar findings across tissues can strengthen biological plausibility, but direct evidence in the relevant tissue and population remains more informative than extrapolation
This distinction is essential for the Keyora Mitochondrial Resilience framework.
It allows multiple evidence streams to be integrated without pretending that every mitochondrial finding is universally interchangeable.
What Does Human Evidence Actually Show About Astaxanthin and Energy-Related Function?
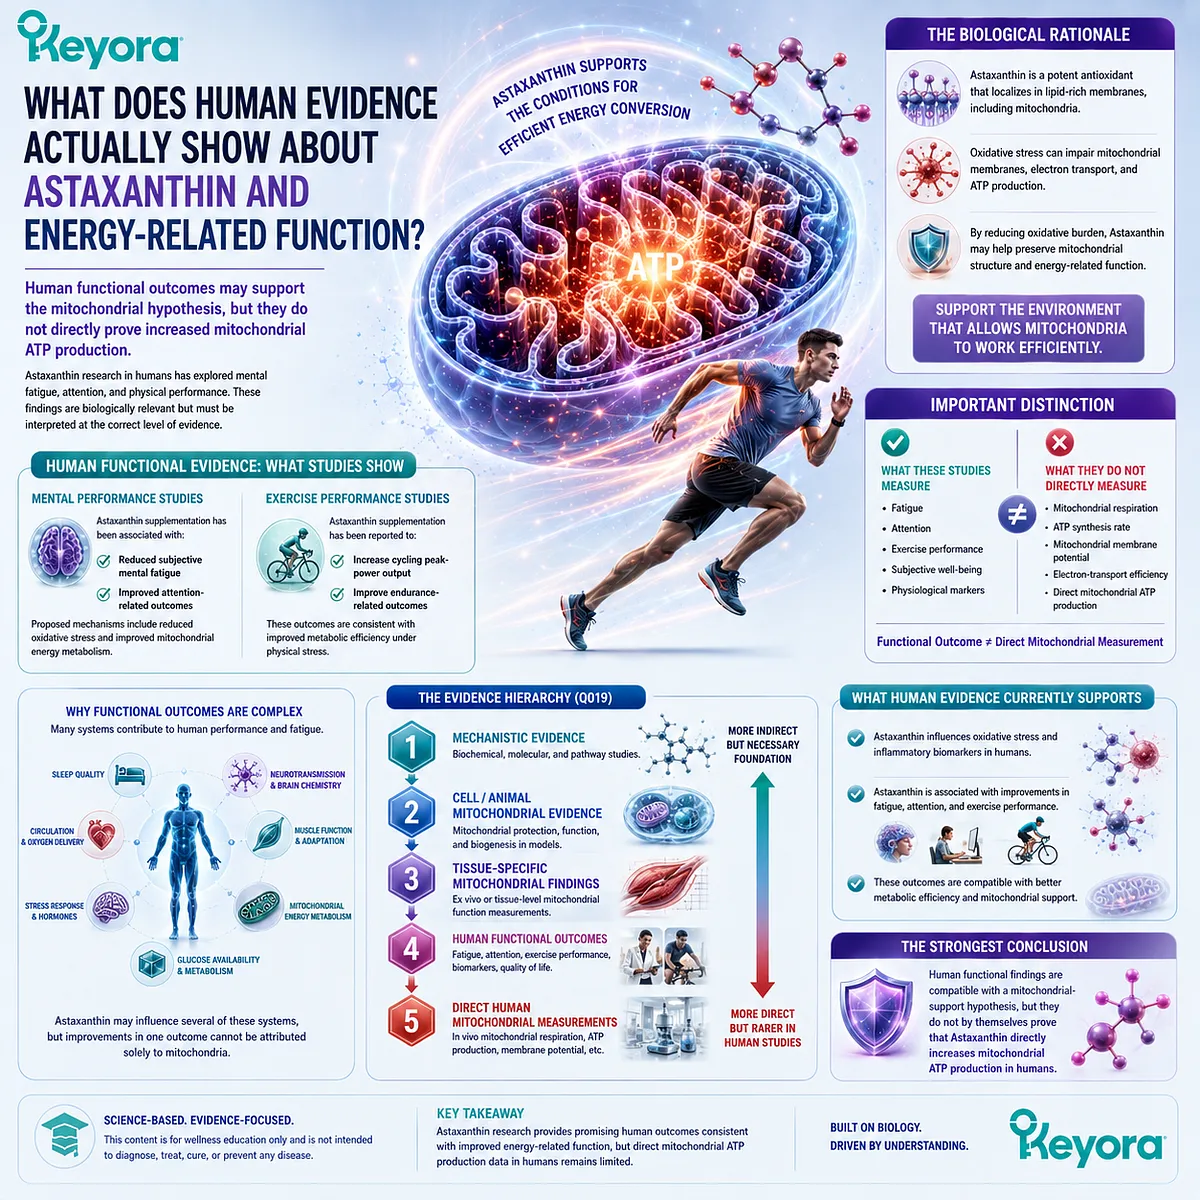
Human functional outcomes may support the mitochondrial hypothesis, but they do not directly prove increased mitochondrial ATP production
The mitochondrial case becomes more complicated when moving from mechanistic studies to human outcomes.
The supplied Astaxanthin source discusses human research related to mental fatigue, attention, and physical performance.
For mental performance, the source describes Astaxanthin supplementation in connection with reduced subjective mental fatigue and improved attention-related outcomes, while proposing reduced oxidative stress and improved mitochondrial energy metabolism as possible mechanisms.
The source also discusses exercise-related research and reports human performance findings such as changes in cycling peak-power output.
These findings are relevant – but they must not be overinterpreted.
A study measuring:
fatigue
or
attention
or
cycling performance
is not automatically a study directly measuring:
-
mitochondrial respiration;
-
ATP synthesis rate;
-
mitochondrial membrane potential;
-
electron-transport efficiency.
That leads to one of the most important evidence rules in Q019:
Functional Outcome ≠ Direct Mitochondrial Measurement
A human participant performing better on an exercise test may be consistent with improved metabolic efficiency, but many physiological systems contribute to performance.
Similarly, reduced mental fatigue can involve sleep, circulation, neurotransmission, stress responses, glucose availability, and multiple other processes in addition to mitochondria.
The evidence hierarchy is therefore:
Mechanistic evidence
↓
Cell / animal mitochondrial evidence
↓
Tissue-specific mitochondrial findings
↓
Human functional outcomes
↓
Direct human mitochondrial measurements
The supplied sources provide meaningful evidence in the middle layers.
They provide much less direct evidence that Astaxanthin supplementation increases mitochondrial ATP production across humans generally.
The strongest conclusion is therefore supportive rather than absolute:
Human functional findings are compatible with a mitochondrial-support hypothesis, but they do not by themselves prove that Astaxanthin directly increases mitochondrial ATP production in humans.
Does Astaxanthin “Boost Mitochondria” – or What Can We Actually Conclude?
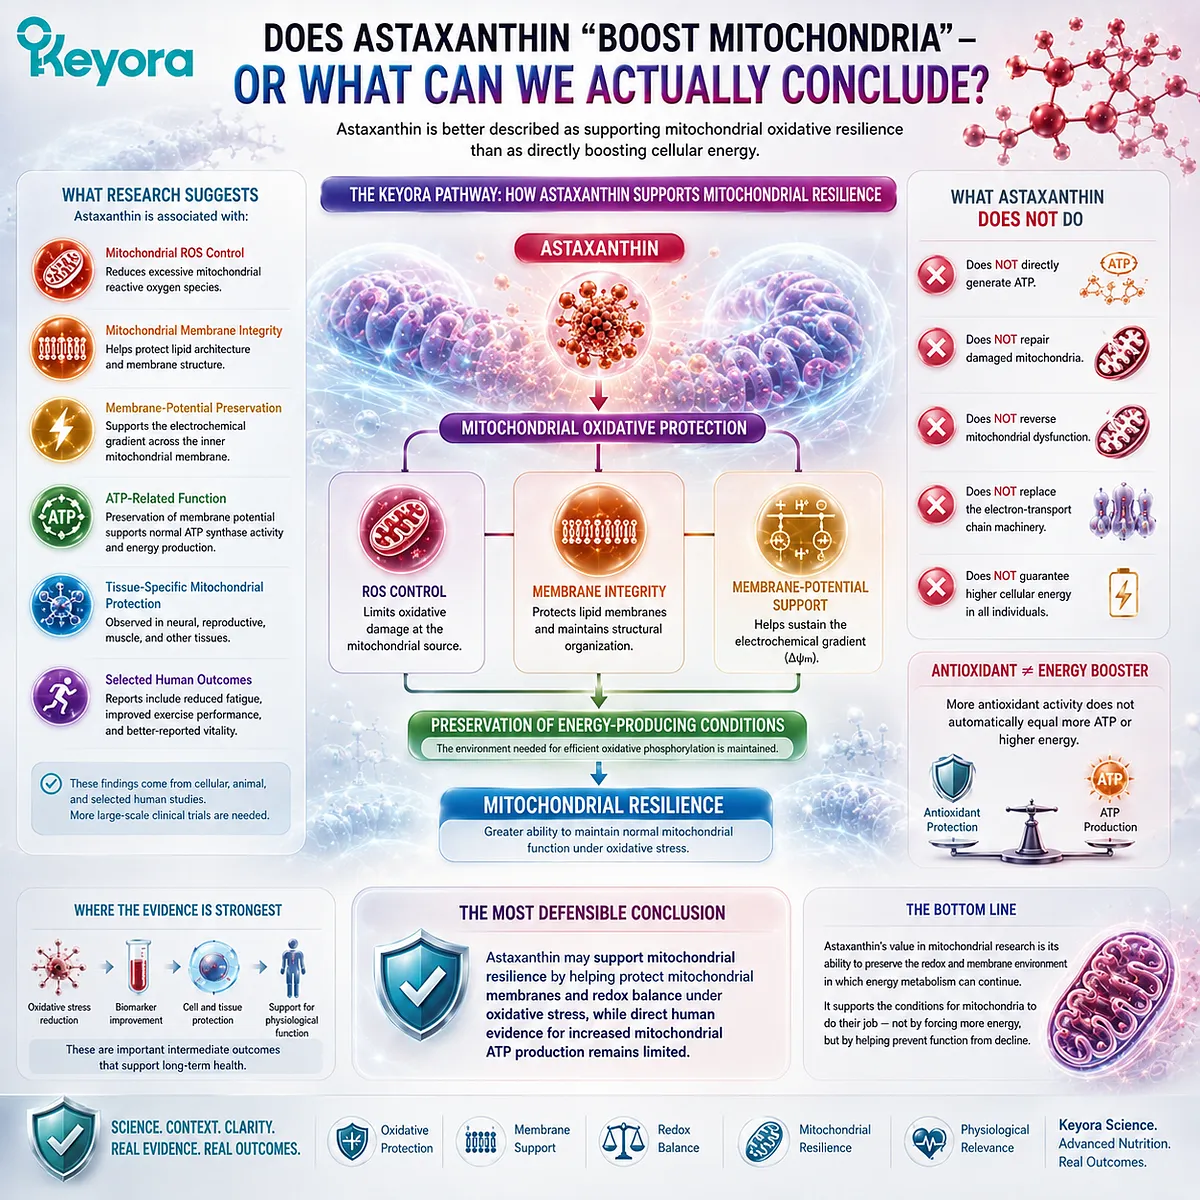
Astaxanthin is better described as supporting mitochondrial oxidative resilience than as directly boosting cellular energy
The current evidence supports a clear but bounded conclusion.
Astaxanthin has a credible mechanistic rationale for supporting mitochondrial resilience under oxidative stress.
The supplied Keyora sources connect Astaxanthin with:
-
mitochondrial ROS control;
-
mitochondrial membrane integrity;
-
membrane-potential preservation;
-
ATP-related function;
-
tissue-specific mitochondrial protection;
-
selected human fatigue and performance outcomes.
But these findings do not establish that Astaxanthin universally “boosts mitochondria.”
They do not justify saying that Astaxanthin:
directly generates ATP
or
repairs damaged mitochondria
or
reverses mitochondrial dysfunction
or
guarantees higher cellular energy
The more evidence-aligned Keyora pathway is:
Astaxanthin
↓
Mitochondrial Oxidative Protection
↓
ROS Control
Membrane Integrity
Membrane-Potential Support
↓
Preservation of Energy-Producing Conditions
↓
Mitochondrial Resilience
Within this framework, Astaxanthin is not an ATP booster.
It is a nutrient being studied for its ability to help preserve the redox and membrane environment in which mitochondrial energy metabolism takes place.
That distinction matters.
It separates a scientifically credible mitochondrial-support argument from a generalized “more antioxidant equals more energy” claim.
The most defensible conclusion is therefore:
Astaxanthin may support mitochondrial resilience by helping protect mitochondrial membranes and redox balance under oxidative stress, while direct human evidence for increased mitochondrial ATP production remains limited.
This article is for educational and informational purposes only. It does not provide medical advice, diagnosis, treatment, cure, prevention, disease outcome claims, hormone restoration claims, fertility outcome claims, or formula-specific clinical efficacy claims.